Saturday, August 30, 2014

"Non-avian dinosaurs" (2)

As I said in the previous post:

The phrase "non-avian dinosaurs" crops up in many articles. What does it mean? As we see below it means Dinosauria minus Aves. Unfortunately, it lumps in the feathered basal paraves with the real dinosaurs such as Tyrannosaurus, under the same label - "non-avian dinosaur". In short, it lumps basal paraves in with actual dinosaurs.

Why is this a problem?
The problem is that when someone makes a statement about "non-avian dinosaurs" we do not know whether they are referring to feathered Paraves (which are feathered) or whether they are referring to actual dinosaurs (which do not have feathers).

For example take a quote like the following:
http://en.wikipedia.org/wiki/Feathered_dinosaur
"it was not until the early 1990s that clearly nonavian dinosaur fossils were discovered with preserved feathers. Today there are more than twenty genera of dinosaurs with fossil feathers, nearly all of which are theropods. "
We cannot tell whether the quote refers just to feathered Paraves or whether it refers to actual dinosaurs. The way it is worded it leaves the impression that there were actually feathered dinosaurs.
So when someone claims that there are many feathered dinosaurs found, they are almost always referring to feathered Paraves which are not actually dinosaurs.
That is why the phrase "non-avian dinosaurs" (or "non-avian theropods") is not nearly precise enough. In fact, it is misleading.

Here is another example, where they are talking only about oviraptors and not actual dinosaurs. But they call them "non-avian theropods".
http://en.wikipedia.org/wiki/Caudipteryx
Because Caudipteryx has clear and unambiguously pennaceous feathers, like modern birds, and because several cladistic analyses have consistently recovered it as a nonavian, oviraptorid, dinosaur, it provided, at the time of its description, the clearest and most succinct evidence that birds evolved from dinosaurs. Lawrence Witmer stated: “The presence of unambiguous feathers in an unambiguously nonavian theropod has the rhetorical impact of an atomic bomb, rendering any doubt about the theropod relationships of birds ludicrous.”[3]

And on the other hand:
When someone does explicitly claim that an actual dinosaur had feathers, it turns out they are not feathers but bristles. (That is a separate subject, covered earlier).


Wednesday, August 27, 2014

"Non-avian dinosaurs"

What does "non-avian dinosaur" mean?

The phrase "non-avian dinosaurs" crops up in many articles. What does it mean? As we see below, it lumps in the basal paraves (the feathered primitive flying and secondarily flightless primitive birds) with the real dinosaurs such as Tyrannosaurus - all of them under the same label - "non-avian dinosaur". In other words, it lumps in basal paraves with actual dinosaurs. 

"Now consider the group consisting of the non-avian dinosaurs (which is what people usually mean by the informal term "dinosaurs''). This is a paraphyletic group, because it can't be defined simply as ``this animal plus all its descendants'', but must be described as one clade minus another: in this case, Dinosauria minus Aves. The ``non-avian dinosaurs'' make up a singly paraphyletic group because only one clade need be omitted from its base definition."

"it was not until the early 1990s that clearly nonavian dinosaur fossils were discovered with preserved feathers. Today there are more than twenty genera of dinosaurs with fossil feathers, nearly all of which are theropods. "
"By the 1990s, most paleontologists considered birds to be surviving dinosaurs and referred to 'non-avian dinosaurs' (all extinct), to distinguish them from birds (aves)."

AND notice these variations:

"Recent studies by Varricchio et al. reveal that males cared for the eggs of troodontids and oviraptorids, so-called "non-avian theropods" of the Cretaceous".

"The smallest non-avialan theropod known from adult specimens is the troodontid Anchiornis huxleyi, at 110 grams in weight and 34 centimeters (1 ft) in length.[3] "

I will talk about why this is a problem in the next post. 

Another claimed "feathered dinosaur" (2)

Continuing the analysis of Kulindadromeus:

http://en.wikipedia.org/wiki/Kulindadromeus
The second type is represented by groups of six or seven downwards projecting up to 1.5 centimetres long filaments, together originating from a base plate. These are present on the upper arm and thigh. They resemble the type 3 feathers of theropods. The base plates are ordered in a hexagonal pattern but do not touch each other.
However the supplementary material tells a different story:

http://www.sciencemag.org/content/suppl/2014/07/23/345.6195.451.DC1/Godefroit.SM.pdf
We considered attempting to describe the feather morphotypes in Kulindadromeus using the nomenclature of Prum et al. (52, 53) or of Xu et al. (21, 22). However, except for our monofilaments (which correspond well to Type 1 in Xu et al.), we could not assign with confidence the other two feather morphotypes in Kulindadromeus to categories described by Prum et al. or Xu et al. Further, fundamental discrepancies between these two previously published nomenclature systems remain to be resolved. Thus we felt that until new fossil material and a synthesis of existing nomenclature systems are available, interpretations of direct homologies between complex feather-types in Kulindadromeus and in Prum et al. or Xu et al. would be premature.
A claim of anything beyond "type 1" filaments (that are actually just bristles) goes beyond the evidence, as confirmed by the supplementary material.

This quote expresses exactly what I am saying:
http://reptilis.net/2014/07/31/new-siberian-ornithischian-and-the-over-feathering-of-dinosaurs-again/
So I find it quite strange and disheartening that Godefroit et al.—despite being fairly objective in their supplementary material—go completely gung-ho in calling these structures feathers.

Tuesday, August 26, 2014

Another claimed "feathered dinosaur"

Let's begin with an accumulation of material about Kulindadromeus:

http://en.wikipedia.org/wiki/Kulindadromeus
Kulindadromeus is a feathered, herbivorous dinosaur, a basal neornithischian from the Jurassic of Russia. Its integument is evidence for the trait being basal to Dinosauria as a whole, rather than just to Coelurosauria, as previously suspected.
Kulindadromeus is significant in that the various specimens show large parts of its integument. This includes imbricated rows of scales on top of its tail and also a covering of scales branching into feather-like structures, which until its discovery were thought to be exclusive to the Theropoda, of the saurischian-line.[5] The feather remains discovered are of three types, adding a level of complexity to the evolution of feathers in dinosaurs.[4] The first type consists of hair-like filaments covering the trunk, neck and head. These are up to three centimetres long and resemble the stage 1 "dino-fuzz" already known from theropods like Sinosauropteryx. The second type is represented by groups of six or seven downwards projecting up to 1.5 centimetres long filaments, together originating from a base plate. These are present on the upper arm and thigh. They resemble the type 3 feathers of theropods. The base plates are ordered in a hexagonal pattern but do not touch each other. The third type is unique. It was found on the upper lower legs and consists of bundles of six or seven ribbon-like structures, up to two centimetres long. Each ribbon is constructed from about ten parallel filaments up to 0.1 millimetres wide.[1]
Godefroit et al. concluded that the filaments earlier reported in Ornithischia, with Psittacosaurus and Tianyulong, could be homologous to the "protofeathers" found in non-avian theropods. With known feather-like structures in pterosaurs, there is evidence for it being basal to Ornithodira.

http://www.sciencemag.org/content/345/6195/451.abstract
A Jurassic ornithischian dinosaur from Siberia with both feathers and scales

  • Paul Spagna1
  •  
    Middle Jurassic to Early Cretaceous deposits from northeastern China have yielded varied theropod dinosaurs bearing feathers. Filamentous integumentary structures have also been described in ornithischian dinosaurs, but whether these filaments can be regarded as part of the evolutionary lineage toward feathers remains controversial. Here we describe a new basal neornithischian dinosaur from the Jurassic of Siberia with small scales around the distal hindlimb, larger imbricated scales around the tail, monofilaments around the head and the thorax, and more complex featherlike structures around the humerus, the femur, and the tibia. The discovery of these branched integumentary structures outside theropods suggests that featherlike structures coexisted with scales and were potentially widespread among the entire dinosaur clade; feathers may thus have been present in the earliest dinosaurs.
    http://news.nationalgeographic.com/news/2014/07/140724-feathered-siberia-dinosaur-scales-science/
    The scales on Kulindadromeus resemble the scaly skin seen on some birds, the study says, which also argues for a deep genetic root linking dinosaurs to birds.
    Two earlier ornithischian dinosaur discoveries, both from China, had hinted that featherlike bristles had covered dinosaurs, notes paleontologist Stephen Brusatte of the United Kingdom's University of Edinburgh.
    "But the new Siberian fossils are the best example yet that some ornithischian [beaked] dinosaurs had feathers, so it wasn't only the theropods that had downy coats," Brusatte says.
    "This does mean that we can now be very confident that feathers weren't just an invention of birds and their closest relatives, but evolved much deeper in dinosaur history," he adds. "I think that the common ancestor of dinosaurs probably had feathers, and that all dinosaurs had some type of feather, just like all mammals have some type of hair."

    http://palaeo.gly.bris.ac.uk/melanosomes/Kulindaimages.html

    http://www.ncbi.nlm.nih.gov/pubmed/19295609

    http://en.wikipedia.org/wiki/Tianyulong

    http://link.springer.com/article/10.1007%2Fs00114-002-0339-6

    http://en.wikipedia.org/wiki/Psittacosaurus

    http://www.theguardian.com/world/2014/jul/24/dinosaur-feathers-siberia-fossil-discovery-herbivore

    http://www.walkingwithdinosaurs.com/news/post/did-triceratops-have-feathers-or-quills/

    http://pterosaurnet.blogspot.ca/2014/01/helpful-background.html

    http://flyingdinosaurs.net/a-z-of-feathered-dinosaurs/


    For reference:
    Stage 1:


    From the supplementary material:
    http://www.sciencemag.org/content/suppl/2014/07/23/345.6195.451.DC1/Godefroit.SM.pdf
    We considered attempting to describe the feather morphotypes in Kulindadromeus using the nomenclature of Prum et al. (52, 53) or of Xu et al. (21, 22). However, except for our monofilaments (which correspond well to Type 1 in Xu et al.), we could not assign with confidence the other two feather morphotypes in Kulindadromeus to categories described by Prum et al. or Xu et al. Further, fundamental discrepancies between these two previously published nomenclature systems remain to be resolved. Thus we felt that until new fossil material and a synthesis of existing nomenclature systems are available, interpretations of direct homologies between complex feather-types in Kulindadromeus and in Prum et al. or Xu et al. would be premature.

     http://www.bbc.com/news/science-environment-28407381
    But Dr Paul Barrett of the Natural History Museum in London, has doubts.
    "Most feathers have a branching structure," he told BBC News.
    "Instead these look like little streamers coming from a central plate. No bird has that structure in any part of its plumage and none of the developmental models that biologists use to understand the evolution of feathers includes a stage that has anything like that kind of anatomy."
    http://news.nationalgeographic.com/news/2014/07/140724-feathered-siberia-dinosaur-scales-science/
    Kulindadromeus adds a whole new dimension to understanding feather evolution, Vinther says, pointing to the fact that the three feather types found as imprints with the fossils are different from ones found on feathered dinosaurs or modern birds.
    What exactly did all these different feathers do? "I don't know; nobody knows for sure," Godefroit says. "These animals couldn't fly, that's all we can tell you."
    http://reptilis.net/2014/07/31/new-siberian-ornithischian-and-the-over-feathering-of-dinosaurs-again/
    So I find it quite strange and disheartening that Godefroit et al.—despite being fairly objective in their supplementary material—go completely gung-ho in calling these structures feathers.

    Wednesday, August 6, 2014

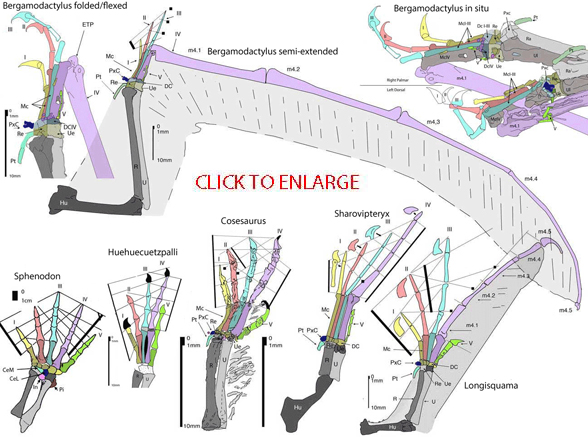
    Hand Transition

    There is a group of researchers and academics (eg. Feduccia et al) that makes a very strong case that birds did not evolve from dinosaurs.

    One important aspect of their argument is the discrepancy in digits (fingers) between dinosaurs and modern birds. The evidence indicates that birds have digits II-III-IV while dinosaurs have I-II-III.

    I agree with the researchers and academics that birds did not evolve from dinosaurs.
    I go a step further and suggest that the ancestors were pterosaurs.
    Pterosaur hands and basal paraves hands are such that a very straightforward transition is possible.


    Note that David Peters make an interesting case for the idea that the Yi qi "styliform element" is a displaced radius and ulna.
    https://pterosaurheresies.wordpress.com/2015/05/03/no-styliform-element-on-yi-qi-thats-just-a-displaced-radius/
    https://pterosaurheresies.wordpress.com/2015/05/04/yi-qi-and-occams-razor/


    Dinosaur hand transition reference:
    https://www.google.ca/url?sa=t&rct=j&q=&esrc=s&source=web&cd=3&cad=rja&uact=8&ved=0CCsQFjAC&url=http%3A%2F%2Fwww.researchgate.net%2Fprofile%2FXing_Xu%2Fpublication%2F240308509_Tracing_the_Evolution_of_Avian_Wing_Digits%2Flinks%2F02e7e537560ae766a3000000.pdf&ei=CZxGVaugLNalyAS1nIDgAg&usg=AFQjCNFdcg3bgYQxu_mVRcztatgns_d_fQ&sig2=PauK8RYVATPAVZvHO0sFwA&bvm=bv.92291466,d.aWw

    Also see the July 30 post.

    http://www.sciencedirect.com/science/article/pii/S0169534702000186
    New studies by Larsson and Wager, and by Feduccia and Nowicki of the embryogenesis of birds undisputedly show Anlagen for five fingers. This has important implications. First, the early presence of digit I, and its later disappearance, indicate that the evolutionary reduction of digits occurred via developmental arrest followed by degeneration. Second, it shows that the digits in the wings of birds develop from Anlagen II–IV. This suggests that the hypothesized descent of birds from theropods might be problematic, because theropods are assumed to have digits I–III.

    Wednesday, July 30, 2014

    Pterosaur fingers


    Pterosaur


    ALTERNATIVES

    https://en.wikipedia.org/wiki/Origin_of_birds#Digit_homology
    The phalangeal count for archosaurs is 2-3-4-5-3


    Thumbs Down
    https://www.researchgate.net/publication/259253962_Thumbs_Down_A_MolecularMorphogenetic_Approach_to_Avian_Digit_Homology
    We argue that limb bud cells that would normally form the digit II condensation proliferate toward a more anterior direction, into the space made physically available by the loss of digit I. This causes the presumptive digit II to leave the Shh activity zone. At the same time its cells do not express hoxD12 (and other posterior digit markers) any more, and therefore its transcriptome becomes characteristic of digit I. Its phalangeal number is reduced--whether due to weaker anterior FGF8 signaling, caused by lower Shh levels that would otherwise stabilize the expression, or because of different hox and downstream gene expression.  

     http://onlinelibrary.wiley.com/enhanced/doi/10.1002/jez.b.22545/#jezb22545-bib-0065
    Thumbs down: a molecular-morphogenetic approach to avian digit homology
    In the initial presentation of the concept, Kundrát et al. (2002) also suggested a mechanism that would be able to derive the Archaeopteryx phalangeal formula from the archosaur one. While the archosaur ground state is thought to be DI(2)–DII(3)–DIII(4)–DIV(5)–DV(3), Archaeopteryx could have DI(2)–DII(3)–DIII(4)–DV(0)–DV(0), but could also be interpreted as DI(0)–DII(2)–DIII(3)–DIV(4)–DV(0). Experiments with molecular signaling pathways in early limb development have shown that modulating interdigital bmp signaling (Dahn and Fallon, 2000) or blocking bmp with a dominant negative receptor (Zou and Niswander, 1996) is able to remove one phalanx from each digit, and therefore a mechanism like that could have caused the archosaur central digits to resemble the Archaeopteryx ones with regard to their phalangeal numbers.


    Pyramid reduction hypothesis

    http://www.cell.com/current-biology/fulltext/S0960-9822(13)00512-5
    The ‘pyramid reduction hypothesis’ assumes II-III-IV identities for neornithine manual digits and postulates the existence of a conservative five-digit pattern with a gradual, bilateral reduction of phalanges and metacarpals in avian evolution [9]. One proposed mechanism postulates that an elevation in peripheral BMPs, signaling factors that modulate cell survival and proliferation [60, 61], drove bilateral medial and lateral digital reduction [9]. This hypothesis is developmentally plausible, and is also consistent with the phalangeal reduction pattern seen in basal birds [9, 23]. However, it predicts that the direct avian ancestor had a five-fingered hand with dominant digits II, III, and IV [9], which is inconsistent with the digital reduction data from basal theropods (e.g., all known basal theropods, including ceratosaurs, have a vestigial digit IV) [5, 62, 63, 64]. In fact, the pyramid reduction hypothesis implies that either birds are not descended from theropod dinosaurs, or that some as yet to be discovered basal theropods were five-fingered with dominant digits II, III, and IV.

    http://www.ncbi.nlm.nih.gov/pubmed/12210116?dopt=Abstract
    We report herein that a pentadactyl developmental pattern is evident in early wing morphogenesis of Gallus (chicken) and Struthio (ostrich). Five avascular zones (spatially predestined locations of contiguous metacarpal and phalangeal aggregation) and four interdigital vascular spaces are established by the regression patterns of autopodial vasculature. Transient vestiges of the first and fifth metacarpals are confirmed histologically and histochemically. They lie within the preaxial-most and postaxial-most avascular zones, respectively.
    These observations reveal conservative patterning of the avian hand and corroborate a II-III-IV metacarpal interpretation, argue for II-III-IV identity of ossified digits in birds, and favour a simple reduction rather than a homeotic [frame] shift in terms of the phenotype expressed by Hox genes in the phylogeny of the avian manus. 
    We suggest that gradual, bilateral reduction of phalanges and metacarpals, via apoptosis mediated by BMP, occurred during the evolution of birds (Pyramid Reduction Hypothesis). This is congruent with the establishment of a central wing axis that became co-opted for coordinated movements.


    https://www.academia.edu/13081883/Pentadactyl_ground_state_of_the_avian_wing
    The issue of the homology of bird fingers with those of pentadactyl amniotes has been a topic of contention for nearly 200 years. Data from the fossil record and phylogenetic systematics ascribe bird digit homologies to digits I, II, and III of pentadactyl amniotes while embryological evidence supports digital homologies of II, III, and IV. Using a molecular marker specific for condensation competent mesenchymal cells, we describe a pentadactyl arrangement of prechondrogenic digital anlagen in the wings of stage 29 chick embryos. Only the middle three anlagen develop into mature fingers. This pattern supports the hypothesis that bird fingers develop from digital anlagen II, III, and IV of pentadactylous amniotes. In addition, this result rejects a model assuming a shift in the primary axis in bird digit development and shows that a prechondrogenic digital anlage has been maintained in the bird lineage for at least 220 million years since the last known pentadactylous ancestor of the lineage. Such a vestige suggests that strong constraints are maintaining a pentadactyl ground state in amniotes.

    https://angeldweb.wordpress.com/2016/07/04/problems-with-dinosaur-to-bird-evolution-the-iii-digits/
    However, this view has remained inconsistent with the accepted early condensation patterns for digit progenitors, which show that the three hand digits of modern adult birds developed from the three middle positions. [14, 7, 9]. Furthermore, the assumption that a single frameshift mutation is capable of shifting Digits I, II III into II, III, IV has been shown to be unreliable given that such mutation reveals no adaptive advantage. Rather numerous frame shifts are required to even create an adaptive advantage, as demonstrated by Alan and other researchers. [15]
    Axis shift hypothesis
    https://www.nature.com/articles/ncomms1437
    Our results support the fossil record, indicating that birds evolved from theropod dinosaurs that lost digits 4 and 5 (Fig. 1a) and is consistent with the overlooked 'axis-shift' hypothesis that proposes the primary axis runs through the digit 3 position in bird wings19,20,21 (Figs 1f and g). 

    Alternative explanations for fingers


    PRH, FS1, FS2, HOH, Thumbs Down, LSH.

    http://www.researchgate.net/publication/259253962_Thumbs_down_a_molecular-morphogenetic_approach_to_avian_digit_homology

    And:
    Very recently Xu and Mackem (2013) introduced a digit reduction scheme called the
    lateral shift hypothesis (LSH). Like the TDH, it follows the II, III, IV
    identification of tetanuran digits, and values the positional criteria over the compositional ones. Unlike the TDH, however, it argues
    that a (partial) homeotic anterior shift took place and that digit IV
    was completely re‐evolved, following in both points the FSH


    Also see:
    http://pterosaurnet.blogspot.ca/2014/07/pterosaur-fingers.html

    https://en.wikipedia.org/wiki/Origin_of_birds#Digit_homology
    The phalangeal count for archosaurs is 2-3-4-5-3

    ALTERNATIVES that are not credible

    PROGENESIS
    https://www.researchgate.net/profile/Tony_Thulborn/publication/43456034_Theropod_dinosaurs_progenesis_and_birds_Homology_of_digits_in_the_manus/links/567631d208ae0ad265c0e321.pdf
    For instance, it is predictable that the loss of digit I from the manus should be simultaneous with loss of a single phalanx from one or more of the three remaining digits: as those losses are attributed to a single cause, the depletion of mesenehyme in the limb bud, they should not occur sequentially.  

    THUMBS DOWN
    https://www.researchgate.net/publication/259253962_Thumbs_Down_A_MolecularMorphogenetic_Approach_to_Avian_Digit_Homology
    We argue that limb bud cells that would normally form the digit II condensation proliferate toward a more anterior direction, into the space made physically available by the loss of digit I. This causes the presumptive digit II to leave the Shh activity zone. At the same time its cells do not express hoxD12 (and other posterior digit markers) any more, and therefore its transcriptome becomes characteristic of digit I.
    Its phalangeal number is reduced--whether due to weaker anterior FGF8 signaling, caused by lower Shh levels that would otherwise stabilize the expression, or because of different hox and downstream gene expression.
    Experiments with molecular signaling pathways in early limb development have shown that  modulating interdigital bmp signaling (Dahn and Fallon, 2000) or blocking bmp with a dominant negative receptor (Zou and Niswander, '96) is able to remove one phalanx from each digit
    A comparison of digits within each limb shows that the posterior forelimb digits are more strongly differentiated than the posterior hindlimb digits, and forelimb digit III exhibits a unique expression of Socs2. 
    References
    https://frontiersinzoology.biomedcentral.com/articles/10.1186/1742-9994-11-33

    https://www.researchgate.net/publication/259253962_Thumbs_Down_A_MolecularMorphogenetic_Approach_to_Avian_Digit_Homology

    https://www.ncbi.nlm.nih.gov/pmc/articles/PMC3986427/

    https://www.researchgate.net/publication/301913740_FANTASY_REALITY_A_Critique_of_Smith_'s_Bird_Origins

    https://www.academia.edu/11078361/Pentadactyl_pattern_of_the_avian_wing_autopodium_and_pyramid_reduction_hypothesis

    https://www.academia.edu/1486957/Transcriptomic_analysis_of_avian_digits_reveals_conserved_and_derived_digit_identities_in_birds

    http://dml.cmnh.org/2000Dec/msg00446.html
    Larry Febo

    https://vargaslab.files.wordpress.com/2009/03/vargasfallon2005b3.pdf

    https://pdfs.semanticscholar.org/c41f/be4e5fdc9b95780eefb7c396351290e43b23.pdf

    https://www.academia.edu/13081883/Pentadactyl_ground_state_of_the_avian_wing

    https://www.researchgate.net/publication/260714882_Tracing_the_Evolution_of_Avian_Wing_Digits
    Xu and Mackem

    http://people.eku.edu/ritchisong/554notes1.html


    Also see:
    https://pterosaurnet.blogspot.ca/2014/07/pterosaur-fingers.html

    Alternately a frameshift explanation:

    http://onlinelibrary.wiley.com/doi/10.1002/jez.b.22545/full
    http://www.researchgate.net/publication/259253962_Thumbs_down_a_molecular-morphogenetic_approach_to_avian_digit_homology
    Avian forelimb digit homology remains one of the standard themes in comparative biology and EvoDevo research. In order to resolve the apparent contradictions between embryological and paleontological evidence a variety of hypotheses have been presented in recent years. The proposals range from excluding birds from the dinosaur clade, to assignments of homology by different criteria, or even assuming a hexadactyl tetrapod limb ground state. At present two approaches prevail: the frame shift hypothesis [FSH] and the pyramid reduction hypothesis [PRH]. While the former postulates a homeotic shift of digit identities, the latter argues for a gradual bilateral reduction of phalanges and digits.
    We argue that limb bud cells that would normally form the digit II condensation proliferate toward a more anterior direction, into the space made physically available by the loss of digit I. This causes the presumptive digit II to leave the Shh activity zone. At the same time its cells do not express hoxD12 (and other posterior digit markers) any more, and therefore its transcriptome becomes characteristic of digit I. Its phalangeal number is reduced—whether due to weaker anterior FGF8 signaling, caused by lower Shh levels that would otherwise stabilize the expression, or because of different hox and downstream gene expression

    Thus the change of the phalangeal formula (as in the PRH) is actually caused by the change of the transcriptome (as in the FSH), which in turn is directly caused by the loss of digit I (probably shh and hoxD mediated).

    At the point when digit I is lost completely, the topological and morphogenetic effect causes the remaining digits to grow more toward anterior and therefore to adopt different phenotypic fates (e.g., Deinonychus).
    The new approach presented here traces the origins of both the
    FSH and the PRH to a common source: the loss of digit I. We
    propose a morphogenetic‐molecular model in which the changingtranscriptome as well as the altered phalanx number in birds are
    direct consequences of the reduction of the anterior‐
    most digit.Because this effect is thought to be triggered once digit I is lost, we
    have dubbed it the thumbs down hypothesis (TDH)
    Also:

    https://www.researchgate.net/publication/261607127_New_developmental_evidence_supports_a_homeotic_frameshift_of_digit_identity_in_the_evolution_of_the_bird_wing


    Arguments against a frameshift in dino to bird:

    http://en.wikipedia.org/wiki/Bilateral_Digit_Reduction#Digit_homology
    However, such frame shifts are rare in amniotes and—to be consistent with the theropod origin of birds—would have had to occur solely in the bird-theropod lineage forelimbs and not the hindlimbs (a condition unknown in any animal).[136] This is called Lateral Digit Reduction (LDR) versus Bilateral Digit Reduction (BDR) (see also Limusaurus[137])
    http://www.pnas.org/content/96/9/5111.full.pdf
    Once this happened, we postulate a frame shift—a homeotic transformation—
    in the developmental identity of the initial condensations:
    Condensation CII developed into digit DI, CIII developed
    into DII, and CIV developed into DIII (Fig. 6C), thus
    conserving a functionally significant mature form within the
    confines of a morphogenetic constraint.
    We are not aware of any other case in which such a conflict between a developmental and a functional constraint in digit reduction existed.

    http://onlinelibrary.wiley.com/doi/10.1002/jez.b.22545/full
    http://www.researchgate.net/publication/259253962_Thumbs_down_a_molecular-morphogenetic_approach_to_avian_digit_homology
    it argues that a (partial) homeotic anterior shift took place and that digit IV was completely re-evolved, following in both points the FSH.

    http://www.cell.com/current-biology/pdf/S0960-9822(13)00512-5.pdf
    Shh levels regulate digit pattern to shift their expression domains
    for the developing hand and the re-emergence of a fully
    functional digit in position 4

    https://vargaslab.files.wordpress.com/2009/03/vargasfallon2005b3.pdf
    Therefore, it must be understood clearly that the absence of a selective advantage for the developmental change in the wing does not imply that it could not have occurred.
    From this point of view, the shift in digital identity could have occurred as a selectively neutral change (phenogenetic drift, according to Weiss and Fullerton, 2000)

    http://frietsongalis.nl/wp-content/uploads/2009/06/Galis-et-al.-2005-J-Exp-Zool-B.pdf
    In addition, a homeotic shift of digits 1, 2, 3 into digits 2, 3, 4 in theropods without further anatomical changes does not appear to lead to an adaptive advantage

    GENERAL:

    http://www.dinosauria.org/docs/oryctos/07_03_campbell.pdf
    Even more revealing is the fact that in the Eichstätt specimen it can be seen that the ginglymoid joint at the end of Metacarpal II is rotated almost 90 degrees, such that in dorsal view it is clear that flexion/extension of Phalanx 1 of Digit II was primarily in the anterior/posterior plane
    Significantly, an anteroposterior flexion/extension of Digit II, even with a sizable ventral component, would have made it the first avian alula, albeit a very primitive one. 
    The basal paraves II digit is basically at right angles to the other two digits. It forms a "primitive alula". It has a quite different structure and function than the dinosaur 1st digit.


    http://www.nature.com/nature/journal/v500/n7463/full/nature12336.html
    Digit loss is defined as the complete loss of all phalanges and the
    metapodial bone; it should be distinguished from digit reduction, in
    which only phalanges are lost3. Digit loss can be adaptive. It reduces the
    mass of the distal limb, and therefore its moment of inertia; this conserves
    energy during running and flying12–14. 


    http://onlinelibrary.wiley.com/doi/10.1002/dvdy.22595/full


    http://onlinelibrary.wiley.com/doi/10.1002/jez.b.22545/full
    http://www.researchgate.net/publication/259253962_Thumbs_down_a_molecular-morphogenetic_approach_to_avian_digit_homology


    https://www.academia.edu/1486957/Transcriptomic_analysis_of_avian_digits_reveals_conserved_and_derived_digit_identities_in_birds
    To discover genes that specifically contribute to the second and third wing digit identities, we performed differential expression analysis of the mRNA-seq data between samples LFb and LFc. We found two genes, Tbx3 and Socs2, with high expression in sample LFc (Supplementary Fig. 9 and Fig. 3a). To our knowledge no studies have been published indicating a role for Socs2 in limb development. ISH confirms its strong expression in the third forelimb digit to the exclusion of all other digits in forelimb and hindlimb(Fig.3b–g). Recently it has been shown that the third forelimb digit has a unique mode of development in birds8. This, combined with our gene expression survey, supports the idea that the third wing digit has a unique derived identity in birds.

    Other references:
    http://www.researchgate.net/publication/222677306_An_old_controversy_solved_bird_embryos_have_five_fingers
    We are therefore left with several scenarios: (1) birds
    descending from archosaurs other than dinosaurs, which
    cannot satisfactorily explain the many similarities
    between birds and theropods; (2) the FSH, for which
    there is as yet no adaptive significance that would
    overcome the evolutionary constraint; and (3) birds
    descending from theropods with digits II–IV, which is
    the most parsimonious evolutionary transition scenario
    but for which there is as yet no fossil evidence.
    AND
    http://www2.gwu.edu/~newsctr/newscenter/research/dinosaur/clark.pdf
    AND
    http://blogs.discovermagazine.com/loom/2009/06/17/of-birds-and-thumbs/#.U-Okefnlp1Y
    AND
    http://genomebiology.com/content/pdf/gb-2011-12-10-130.pdf
    AND
    http://www.sciencedaily.com/releases/2011/09/110904140359.htm
    AND
    http://www.ncbi.nlm.nih.gov/pmc/articles/PMC3333764/

    Friday, July 25, 2014

    Scansoriopteryx

    Scansoriopteryx is an excellent example of a transitional on the lineage from pterosaur to primitive bird. It is a member of basal Paraves.

    Feduccia and Czerkas article:

    ORIGINAL ARTICLE
    Jurassic archosaur is a non-dinosaurian bird
    Stephen A. Czerkas •Alan Feduccia
    Received: 17 April 2014 / Revised: 4 June 2014 / Accepted: 13 June 2014 / Published online: 9 July 2014
    ÓDt. Ornithologen-Gesellschaft e.V. 2014
    Abstract Re-examination utilizing Keyence 3D digital
    microscopy and low angled illumination of the fossil
    Scansoriopteryx, a problematic sparrow-size pre-Archae-
    opteryx specimen from the Jurassic Daohugou Biotas, pro-
    vides new evidence which challenges the widely accepted
    hypothesis that birds are derived from dinosaurs in which
    avian flight originated from cursorial forms. Contrary to
    previous interpretations in which S
    The re-examination of a sparrow-sized fossil [Scansoriopteryx] from China challenges the commonly held belief that birds evolved from ground-dwelling theropod dinosaurs that gained the ability to fly. The birdlike fossil is actually not a dinosaur, as previously thought, but much rather the remains of a tiny tree-climbing animal that could glide, say American researchers Stephen Czerkas of the Dinosaur Museum in Blanding, Utah, and Alan Feduccia of the University of North Carolina. The study appears in Springer’s Journal of Ornithology.

    Feduccia added, “Instead of regarding birds as deriving from dinosaurs, Scansoriopteryx reinstates the validity of regarding them as a separate class uniquely avian and non-dinosaurian.”

    ELONGATE OUTER FINGER

    Jurassic archosaur is a non-dinosaurian bird
    Stephen A. Czerkas, Alan Feduccia
    Re-examination utilizing Keyence 3D digital microscopy and low angled illumination of the fossil Scansoriopteryx, a problematic sparrow-size pre-Archaeopteryx specimen from the Jurassic Daohugou Biotas, provides new evidence which challenges the widely accepted hypothesis that birds are derived from dinosaurs in which avian flight originated from cursorial forms. Contrary to previous interpretations in which Scansoriopteryx was considered to be a coelurosaurian theropod dinosaur, the absence of fundamental dinosaurian characteristics demonstrates that it was not derived from a dinosaurian ancestry and should not be considered as a theropod dinosaur. Furthermore, the combination in which highly plesiomorphic non-dinosaurian traits are retained along with highly derived features, yet only the beginnings of salient birdlike characteristics, indicates that the basal origins of Aves stemmed from outside the Dinosauria and further back to basal archosaurs. Impressions of primitive elongate feathers on the forelimbs and hindlimbs suggest that Scansoriopteryx represents a basal form of “tetrapteryx” in which incipient aerodynamics involving parachuting or gliding was possible. Along with unique adaptations for an arboreal lifestyle, Scansoriopteryx fulfills predictions from the early twentieth century that the ancestors of birds did not evolve from dinosaurs, and instead were derived from earlier arboreal archosaurs which originated flight according to the traditional trees-down scenario.
    The most unusual feature is the extremely elongate outer finger, considered here to be digit IV as in Aves (Capek et al. 2013). It is the longest manual digit whereas the middle digit in theropods is the longest.

    http://dinosaur-museum.org/featheredinosaurs/arboreal_maniraptoran.pdf
    Scansoriopteryx heilmanni is the only known
    saurischian, or theropod, which has the third digit of the manus elongated to nearly twice that of the second digit. 
    http://www.labnews.co.uk/news/new-finding-challenges-belief-dinosaurs-evolved-from-birds
    The investigations – published in Journal of Ornithology – found a combination of plesiomorphic or ancestral non-dinosaurian traits along with highly derived unambiguous birdlike features. The researchers specifically note the primitive elongated feathers on the fore- and hind limbs, suggesting Scansoriopteryx is an ancestral form of early birds that had mastered basic aerodynamic manoeuvres of parachuting or gliding from trees.
    These findings fulfil a prediction first made in the 1900s that the ancestors of birds didn’t evolve from dinosaurs, but instead from earlier arboreal archosaurs which originated flight according to the tree-down scenario. These small tree-dwelling archosaurs had improved ability to fly, with feathers that enabled them to at least glide. This ‘tree-down’ view is in contrast with the ‘ground-up’ view many palaeontologists side with.
    “Instead of regarding birds as deriving from dinosaurs, Scansoriopteryx reinstates the validity of regarding them as a separate class uniquely avian and non-dinosaurian,” said Alan Feduccia.
    Pterosaur fingers: 
    http://www.reptileevolution.com/pterosaur-wings.htm


    CAUDAL RODS

     http://www.sci-news.com/paleontology/science-scansoriopteryx-hypothesis-birds-evolved-dinosaurs-02059.html
    The techniques made it possible to interpret the natural contours of the bones. Many aspects of the [Scansoriopteryx] fossil’s pelvis, forelimbs, hind limbs, and tail were confirmed, while it was discovered that it had elongated tendons along its tail vertebrae similar to Velociraptor.
    http://onlinelibrary.wiley.com/doi/10.1111/1755-6724.12009/abstract

    In the tails of dromaeosaurids dinosaurs and rhamphorhynchid pterosaurs, elongate osteological rods extend anteriorly from the chevrons and the prezygapophyses. These caudal rods are positioned in parallel and are stacked dorsoventrally.

    http://pterosaur-net.blogspot.ca/2013/01/guest-post-dragon-tails-what-pterosaurs.html
    The tail of Deinonychus and its raptor relatives is bizarre, but it is not (as Professor Ostrom himself realized) unique. Among all known vertebrates, a similar tail anatomy has evolved in one other group [rhamphorhynchid pterosaurs].
    Consider the below images of a tail of a Bambiraptor and of a Velociraptor. Both are dromaeosaurids with caudal-rod bearing tails and both are fully articulated.

    ACETABULUM

    http://www.aoucospubs.org/doi/full/10.1525/auk.2013.130.1.1
    A partially closed acetabulum is seen in basal archosaurs and
    is characteristic of the scansoriopterids and Jurassic feathered
    forms such as Anchiornis
    initially described as near Aves by Xu et al. (2009).
    http://en.wikipedia.org/wiki/Scansoriopteryx
    Scansoriopteryx also lacks a fully perforated acetabulum, the hole in the hip socket which is a key characteristic of Dinosauria and has traditionally been used to define the group. 
    http://dinosaur-museum.org/featheredinosaurs/arboreal_maniraptoran.pdf
    Scansoriopteryx is clearly more primitive
    than Archaeopteryx in many respects such as its
    saurischian-style pelvis which has remarkably short
    pubes; elongate and robust ischia; and
    comparatively small pubic peduncles. These
    primitive features further suggest that the nearly
    closed acetabulum is not a reversal, but a true
    plesiomorphic condition.

    http://en.wikipedia.org/wiki/Pterosaur
    Pterosaur's hip sockets are oriented facing slightly upwards, and the head of the femur (thigh bone) is only moderately inward facing, suggesting that pterosaurs had a semi-erect stance. It would have been possible to lift the thigh into a horizontal position during flight as gliding lizards do.

    GENERAL

    http://en.wikipedia.org/wiki/Scansoriopterygidae
    Scansoriopteryx (and its likely synonym Epidendrosaurus) was the first non-avian dinosaur found that had clear adaptations to an arboreal or semi-arboreal lifestyle–it is likely that they spent much of their time in trees. Both specimens showed features indicating they were juveniles, which made it difficult to determine their exact relationship to other non-avian dinosaurs and birds. It was not until the description of Epidexipteryx in 2008 that an adult specimen was known.
    The scansoriopterygids would have lived alongside synapsids such as the aquatic Castorocauda and arboreal gliding mammal Volaticotherium, the rhamphorhynchoid pterosaurs Jeholopterus and Pterorhynchus, as well as a diverse range of insect life (including mayflies and beetles) and several species of salamander.[14][15]
    A monophyletic Scansoriopterygidae was recovered by Godefroit et al. (2013); the authors found scansoriopterygids to be basalmost members of Paraves and the sister group to the clade containing Avialae and Deinonychosauria.[9] Agnolín and Novas (2013) recovered scansoriopterygids as non-paravian maniraptorans and the sister group to Oviraptorosauria.[10]

    http://dinosaur-museum.org/featheredinosaurs/arboreal_maniraptoran.pdf
    Scansoriopteryx heilmanni is the only known
    saurischian, or theropod, which has the third digit
    of the manus elongated to nearly twice that of the
    second digit. Scansoriopteryx closely resembles
    Archaeopteryx, but differs in the following: a
    definite contact between an elongate ventral process
    of the postorbital and the ascending process of the
    jugal; the lower jaw is equipped with a large
    fenestra; the tail has a greater development in the
    articulation of the zygapophyses. The pelvis is
    similar to that of Archaeopteryx in having the same
    number of sacrals and general shape of the ilia,
    but
    differs in having a small, unexpanded pubic
    peduncle; a significantly short pubis which is not
    retroverted; longer ischia; and an acetabulum which
    is not entirely perforated.
    Scansoriopteryx is clearly more primitive
    than Archaeopteryx in many respects such as its
    saurischian-style pelvis which has remarkably short
    pubes; elongate and robust ischia; and
    comparatively small pubic peduncles. These
    primitive features further suggest that the nearly
    closed acetabulum is not a reversal, but a true
    plesiomorphic condition.


    http://www.researchgate.net/publication/259438884_Agnoln_and_Novas._2013._Avian_ancestors
    It is important to mention that scansoriopterygids retained a caudoventrally oriented glenoid, a subrectangular coracoid with reduced biceps tubercle, and a distally fan-shaped scapular blade, all representing plesiomorphic character states in respect to paravians.
    Agnolin and Novas provide no support for their assertion that scansoriopterygids had a caudoventrally oriented glenoid.
    http://www.researchgate.net/publicat...vian_ancestors
    In Figure 5.2 they diagram other taxa but not scansoriopteryids. 

    In the published material by those who have analyzed the fossils, I see no mention of a caudoventrally oriented glenoid. (If anyone does see a mention, please give us the link and copy and paste please). 
    https://bio.unc.edu/files/2011/04/Jo...logy-20141.pdf
    http://www.dinosaur-museum.org/feath...niraptoran.pdf


    http://en.wikipedia.org/wiki/Scansoriopteryx
    Zhang et al. also noted that the foot of Epidendrosaurus is unique among non-avian theropods. While the Epidendrosaurus specimen does not preserve a reversed hallux, the backward-facing toe seen in modern perching birds, its foot was very similar in construction to more primitive perching birds like Cathayornis and Longipteryx. These adaptations for grasping ability in all four limbs makes it likely that Epidendrosaurus spent a significant amount of time living in trees.

    Riddle of the Feathered Dragons
    Page 150
    The [Scansoriopteryx] pelvis is still like that of a reptile (as opposed to a theropod) 

    http://link.springer.com/article/10.1007%2Fs10336-014-1098-9#page-1
    the head of [Scansoriopteryx] femur lacks a distinctive neck and is instead more proximally oriented as in reptiles with sprawling limbs


    The reason that the dino to bird folk are confused about this, is that they see the "correction" made at the knee (to make the stance "erect") in basal paraves and birds, and equate this "erect" stance with the quite different "erect" stance of dinosaurs.


    http://books.google.ca/books?id=Z0YWn5F9sWkC&pg=PA46&lpg=PA46&dq=parasagittal+gait&source=bl&ots=5IpEhI42X4&sig=zVn7UBHxK7EYwqz95O7uGIjrIuI&hl=en&sa=X&ei=vLxsVO3cIsOOiwK3mICYBw&ved=0CDwQ6AEwBQ#v=onepage&q=parasagittal%20gait&f=false
    He also pointed out the distinction between a parasagittal gait and a sprawling gait, later understood in terms of fundamentally different mechanics.
    Note the two different meanings:
    http://en.wikipedia.org/wiki/Sagittal_plane
    The term parasagittal is used to describe any plane parallel to the sagittal plane.
    http://evolutionwiki.org/wiki/Parasagittal

    Parasagittal refers to a gait in which the legs are oriented entirely under the body, like columns. Seen in mammals, and birds.

    http://dml.cmnh.org/2008Sep/msg00563.html
    Avialan characters of scansoriopterygids include- - Hyposphene -hypantrum articulations in trunk vertebrae absent (according to Senter).
    Very interesting thoughts from Andrea Cau:

    http://theropoda.blogspot.ca/2012/07/il-ritorno-del-paraviano-pterosauro.html
    In an old post, I have argued, along with Lukas Panzarin, the hypothesis that the highly unorthodox Scansoriopterygidae are of theropodi "pterosaur-like" , converging with small pterosaurs grade rhamphorhynchoide, as they have a short skull, tall and with teeth prominent and projected rostrally, forelegs stretched, the outer finger of the hand hypertrophic but apparently unsuitable to prehension (the penultimate phalanx is not significantly longer than the other), the possible (even if you need a confirmation) of a track patagium nell'olotipo of Scansoriopteryx , attached to the third finger of the hand instead of showing the obvious feathering inserted the second finger as in other maniraptori. The recently described rhamphorhynchoide German Bellubrunnus (Hone et al. 2012) shows a tail very similar to that of Scansoriopteryx . Randomness? Or yet another evidence of convergent evolution? It should be emphasized that the tail of rhamphorhynchidi derivatives is very similar to that of dromaeosauridi derivative, while that of Bellubrunnus is more similar to that of the basal paraviani, such as scansoriopterygidi. Perhaps, the two lineages developed their tails like follow similar evolutionary trajectories, which Scansoriopteryx and Bellubrunnus are both intermediate stages. Although I agree that it is very risky to postulate such a narrow adaptive convergence between baseline and dromaeosauridi rhamphorhynchidi (but Microraptor is potentially arboreal and planatore , then ecologically similar, if not to a flying animal, at least in the same region adaptive in that would place the scansoriopterygidi planatori) I consider it possible that the still little-known faunas of the Middle Jurassic basal paraviani might reserve surprises in the future.
    If the third finger of hypertrophic Scansoriopteryx is already so stretched in the sample holotype, which is very immature, why not imagine that in the adult finger that was even longer? And if so, what good would such an extended finger? Perhaps to support a patagium, especially if it was confirmed the absence of flight feathers in the wing of Epidexipteryx ?
    I admit the many "ifs", but also the many enigmatic aspects of scansoriopterygidi, which probably require explanations heterodox: the assumptions are born so reckless ...
    http://scienceblogs.com/tetrapodzoology/2008/10/23/epidexipteryx-at-last/
    In my large-scale analysis of theropods (in preparation), Scansoriopterygidae are placed sligtly more basal than Avialae: they’re basal paravians, sister-group of Eumaniraptora (Avialae+Deinonychosauria). This different position explains more the “incisivosaur-like” skull and the absence of some pelvic features widespread among basal avialans, dromaeosaurids and troodontids (in particular the scapular, ischial and pubic features).
    In my blog, I suggested an alternative and very heterodox interpretation of Scansoriopterygids: given the absence of evidence for remiges in Epidexipteryx, is it possible that the “feather impressions” seen in the forelimb of the “Scansoriopteryx heilmanni specimen” are not feathers, but a different tegument: it is interesting to note that in remige-bearing maniraptorans, the remiges are inserted on the second finger, whereas in Scasoriopteryx these impression are close to the hyper-elongated third finger. This very long lateral finger is similar to the pterosaurian fourth digit. So, it is possible that the “feather impressions” of Scansoriopteryx were remnant of a patagium. In my opinion, the presence of this structure may explain the elongation of the lateral digit in these small theropods better than the Aye-Aye hypothesis.
    2015:
    http://phenomena.nationalgeographic.com/2015/04/29/chinese-dinosaur-had-bat-like-wings-and-feathers/
    These wings were mutually exclusive: dinosaur or pterosaur, feathery or leathery. But Yi went for both options! It had membrane wings with a feathery covering on the leading edge. It shows that at least some dinosaurs had independently evolved the same kind of wings as pterosaurs—an extraordinary example of convergent evolution.
    http://blogs.scientificamerican.com/tetrapod-zoology/2015/05/05/yi-qi-is-neat/
    Membranous-winged scansoriopterygids were predicted in 2008. Moving on, there are several neat things that I think should be discussed here (scarcely none of which have been mentioned in existing online discussions of this find). The first one is that the concept of a scansoriopterygid with gliding membranes is (while radical and shocking) not novel if you’ve been paying attention.Exactly such a creature was predicted by my colleague Andrea Cau (and illustrated by excellent palaeoartist Lukas Pankarin) way back in October 2008 after the publication of Epidexipteryx* (Zhang et al. 2008). Like Yi qi and other scansoriopterygids, Epidexipteryx lacks vaned feathers yet has a hyper-long digit that looks suitable – Andrea proposed – for the support of a patagial membrane. Yi qi is, therefore, yet another of those fossil animals predicted to exist prior to its discovery. SpecBio fans might like to know that C. M. Kosemen took this suggestion and ran with it, but that’s a story for another time.

    http://dinosaur-museum.org/featheredinosaurs/Are_Birds_Really_Dinosaurs.pdf
    Had Scansoriopteryx been discovered before the use of cladistics became so prevalent some two decades ago, the cursorial theory of how birds evolved from theropod dinosaurs could not have progressed as it has. Scansoriopteryx is known from strata believed to be from the Middle Jurassic, possibly 165 to 180 million years ago, and much older than when Archaeopteryx is known to have lived during the Late
    Jurassic. So there is no time paradox in its being ancestral to birds, as there is for dromaeosaurs of other bird-like dinosaurs. Scansoriopteryx simply does not represent a ground dwelling dinosaur, but it clearly does have a significant ability for climbing while at the same time is not as well developed for flight as was Archaeopteryx. The shoulder/chest complex of the scapula and coracoid are more primitive than
    that of Archaeopteryx. The furcula is not present, but is instead represented by separate clavicles.

    http://dinosaur-museum.org/featheredinosaurs/arboreal_maniraptoran.pdf
    The systematic description of Scansoriopteryx
    depends upon whether certain characters are
    considered as truly plesiomorphic, or as derived
    reversals that only resemble primitive conditions
    secondarily. The main distinction between the two
    interpretations is that Scansoriopteryx was derived
    either from a pre-theropod saurischian [archosaur] ancestor, or
    from a theropod. The first scenario suggests that
    the ancestral forms which led to Scansoriopteryx
    were basal saurischians from the Middle Triassic,
    or earlier, before theropods had appeared. The
    second option would suggest that Scansoriopteryx
    appeared much later in time from a theropod lineage
    which, in becoming arboreal, developed massive
    reversals secondarily resembling primitive
    characteristics. The basal saurischian relationship
    is seen here as being the more parsimonious
    interpretation. 
    The passage above is very good, but there is no reason to think the ancestor was a saurischian dinosaur. It was not any kind of dinosaur. It was actually a pterosaur.


    http://www.nature.com/nature/journal/v498/n7454/full/nature12168.html

    Three main references:

    http://www.ivpp.ac.cn/qt/papers/201206/P020120604508520389814.pdf (2002)
    A juvenile coelurosaurian theropod [Epidendrosaurus] from China indicates arboreal habits
    http://dinosaur-museum.org/featheredinosaurs/arboreal_maniraptoran.pdf

    http://link.springer.com/article/10.1007/s10336-014-1098-9/fulltext.html  (2014)


    Epidexipteryx

    http://en.wikipedia.org/wiki/Epidexipteryx

    The skull of Epidexipteryx is also unique in a number of features, and bears an overall similarity to the skull of Sapeornis, oviraptorosaurs and, to a lesser extent, therizinosauroids. It had teeth only in the front of the jaws, with unusually long front teeth angled forward, a feature only seen in Masiakasaurus among other theropods. The rest of the skeleton bore an overall similarity to the possibly closely related Scansoriopteryx, including a hip configuration unusual among other dinosaurs: the pubis was shorter than the ischium, and the ischium itself was expanded towards the tip. The tail of Epidexipteryx also bore unusual vertebrae towards the tip which resembled the feather-anchoring pygostyle of modern birds and some oviraptorosaurs.[2]